
INTRODUCTION
Heat stress (HS) is a major challenge in swine production, particularly for lactating sows, as it negatively affects overall reproductive performance [1,2]. High ambient temperatures interfere with thermoregulation, leading to increased respiration rates, metabolic acidosis, and reduced voluntary feed intake resulting in insufficient nutrients available for milk production [3]. The decline in feed consumption and metabolic activity is a natural mechanism to lower metabolic heat production [4]. These factors collectively lead to economic losses and reduced productivity in swine operations. Therefore, effective nutritional strategies to mitigate HS effects in lactating sows are essential to maintain optimal sow and litter performance.
Among various strategies, feed form is an important factor influencing nutrient utilization and sow productivity [5]. The mash diet is a common feed type for lactating sows, primarily because it is cost-effective, requires minimal processing, and is easy to produce [5,6]. However, during periods of HS, lactating sows face additional physiological stress and reduced feed intake, making it challenging to meet their elevated nutritional demands through mash diets alone. In this context, pelleted diets, though more expensive, may provide tangible benefits. They improve feed intake and nutrient density due to increased palatability, reduced wastage, enhanced hygienic quality, and prevention of selective feeding [7–9]. These attributes are particularly valuable under HS conditions, where maintaining high feed intake and energy availability is crucial for sustaining sow and litter performance [7].
Despite their benefits, pelleted feeds also have limitations. The pelleting process reduces particle size and increases starch gelatinization, leading to faster digestion and higher gastric acid secretion, which may predispose sows to gastric ulcers [10,11]. This risk is exacerbated during HS, when digestive health is more vulnerable [11]. To address this, sodium bicarbonate (NaHCO₃) supplementation has been explored as a dietary buffer that helps stabilize gastric pH and reduce acidity [12]. Moreover, NaHCO₃ increases dietary electrolyte balance (dEB), calculated as Na + K – Cl (mEq/kg), which plays a crucial role in maintaining acid-base equilibrium during HS [13,14]. A positive dEB has been shown to improve sow performance and support a healthier digestive environment, possibly by modifying gut microbiota composition [6,15,16]. Given these considerations, the combination of pelleted feed and sodium bicarbonate supplementation may offer synergistic advantages. While pelleted feeds enhance feed intake and nutrient utilization, sodium bicarbonate buffers gastric pH and improves dEB, potentially reducing stress and supporting gut integrity. We hypothesized that the synergistic effect of pelleted feed and higher dEB, achieved through sodium bicarbonate supplementation, may alleviate the risk of gastric ulcers by promoting consistent feed intake, stabilizing gastric pH, and enhancing mucosal protection. Thus, the objective of this study was to evaluate the effects of feed form (mash vs. pellet) and dEB levels (230 mEq/kg vs. 290 mEq/kg) on sow and litter performance, nutrient digestibility, milk composition, inflammatory cytokines, antioxidant levels, gut integrity, hair cortisol, salivary pH, and gut microbiota diversity under HS conditions.
MATERIALS AND METHODS
The Kangwon National University Institutional Animal Care and Use Committee approved all protocols involving animal use, care and handling (protocol, KW-240722-4). The NaHCO3 used in the present study was purchased from (SOMA) with purity ≥ 99%.
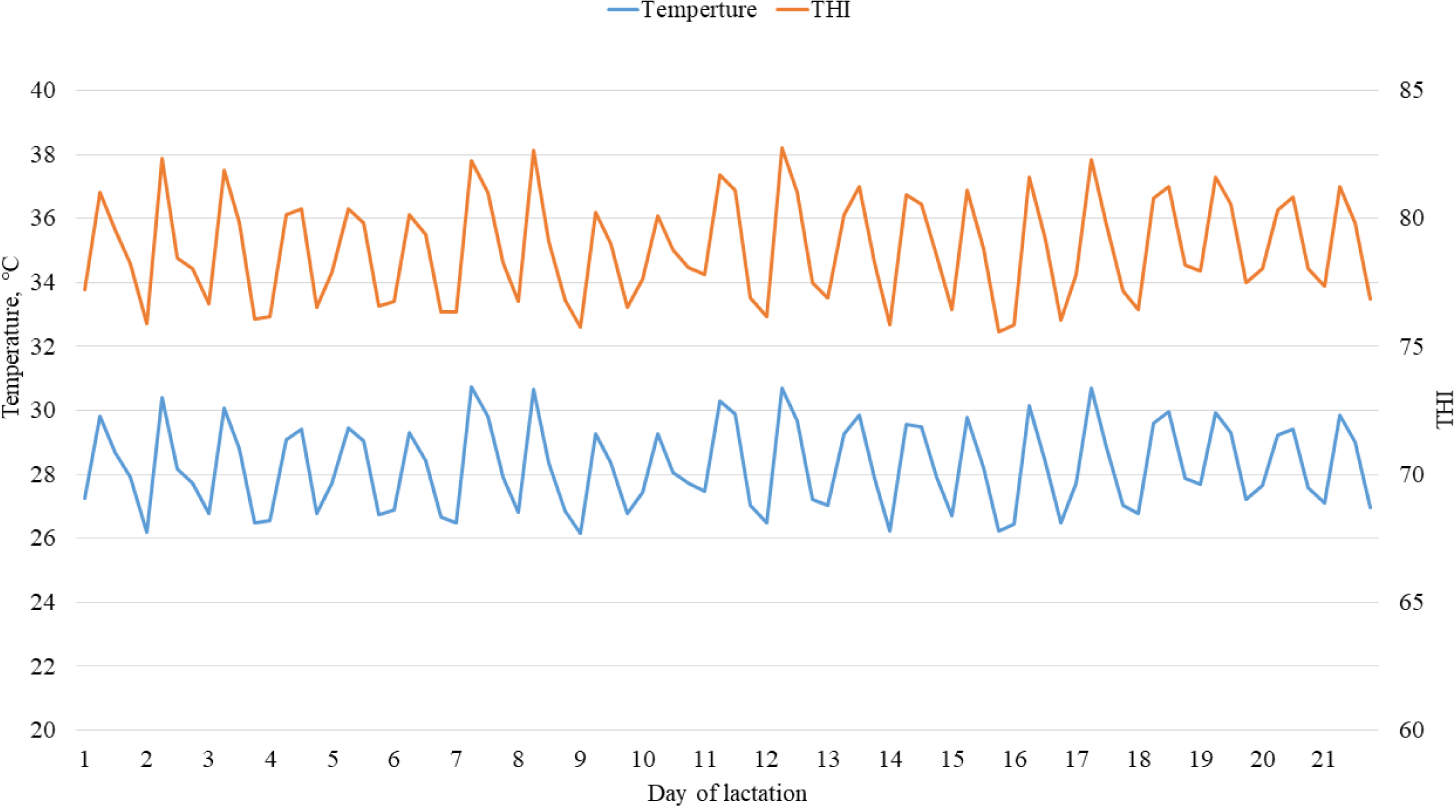
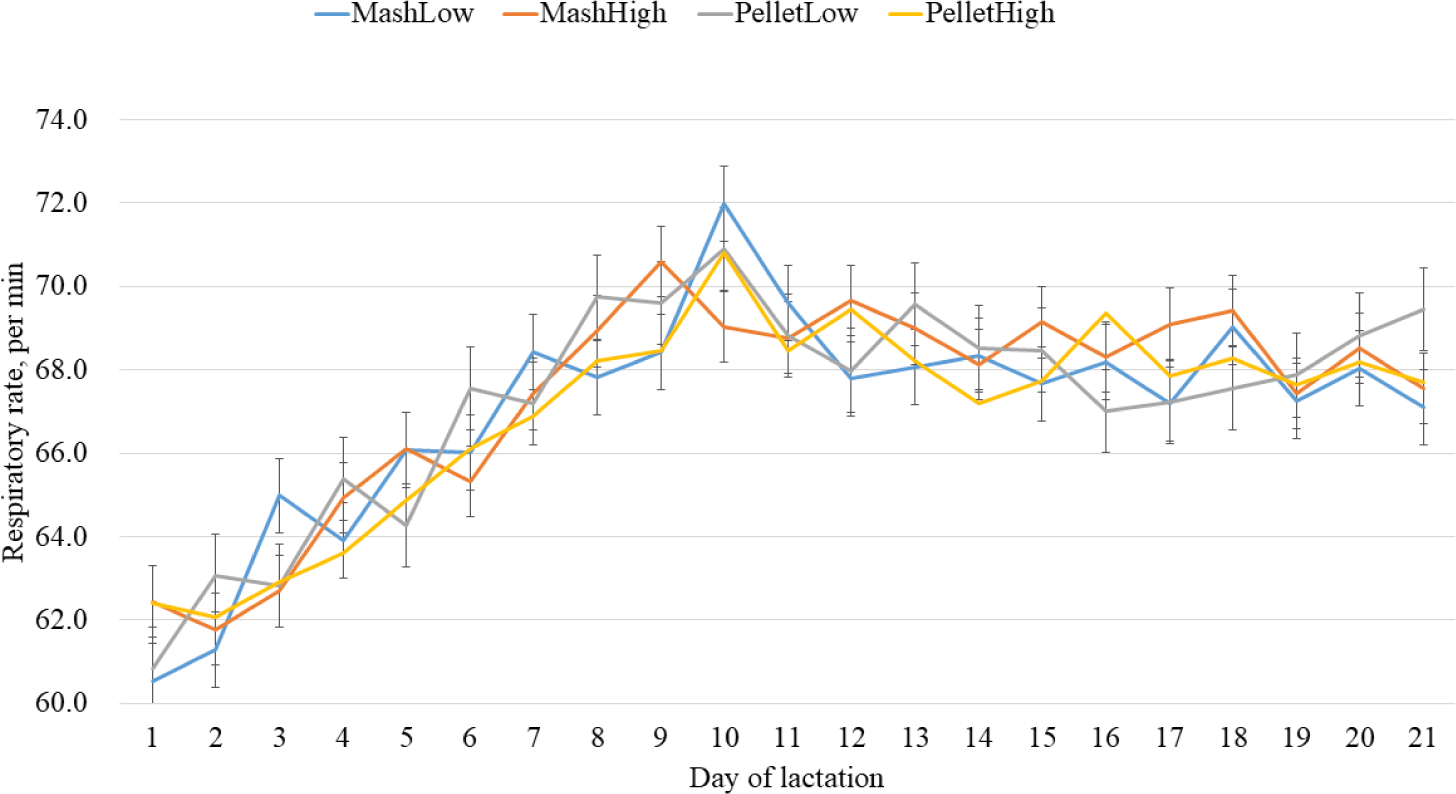
Forty multiparous sows (Landrace × Yorkshire; average initial body weight of 241.83 ± 16 kg) at d 112 of lactation were exposed to HS with an average temperature of 28.25°C. The 21-day (parturition-weaning) experiment was carried out during the summer period of August in Haman-gun, Gyeongsang province, South Korea. The sows were randomly distributed to four treatment diets based on parity in a completely randomized design with 10 pigs per replicate and 1 pig per replicate per head as a 2 × 2 factorial arrangement with 2 feed forms (mash and pellet) and 2 dEB levels (low/230 mEq/kg and high/290 mEq/kg). The treatments include (1) mash diet + 230 mEq/kg (Mlow), (2) mash diet + 290 mEq/kg (Mhigh), (3) pellet diet + 230 mEq/kg (Plow), and (4) pellet diet + 290 mEq/kg (Phigh). Sows were fed every morning and evening, with a feed intake of 2.5 kg per day during gestation. After farrowing, the allowance was gradually increased by 1 kg per day until reaching the maximum limit. All diets were formulated using corn and soybean meal to meet or exceed the nutrient recommendations of NRC [17], AOAC [18] (Table 1) in accordance with a lactating sow feeding program. All precautions were taken to ensure the reduced dEB does not compromise animal health and welfare as shown in the results. Sows were housed in individual farrowing crates (2.14 × 2.15 m), each with designated spaces (2.14 × 2.15 m) on both sides for newborn piglets. Heat lamps were provided to keep the piglets warm. Standard management procedures, including teeth clipping, tail docking, ear notching, and subcutaneous iron dextran injections (1 mL per piglet) within 24 hours of birth, were followed. Sows had unrestricted access to water throughout the experiment, while piglets were not provided with creep feed. Environmental factors, including temperature and humidity, were monitored every five minutes using Tenmars temperature/humidity data loggers (TM-305U, Tenmars Electronics), which were positioned at the level of the sow’s head. The data loggers measured temperature with a tolerance of ± 0.5°C (resolution: 0.02°C) and humidity with an accuracy of ± 3.4% (resolution: 0.2%). The temperature humidity index (THI) was calculated as THI = temperature – [0.55 – (0.0055 × humidity)] × (temperature – 14.5), and the THI and room temperature are shown in Figs. 1 and 2. The THI ranged from 75.58 to 82.76 during the experimental period. Respiratory rates shown in Fig. 3 were measured by observing flank movements over 60 second period and expressed as breaths per minute at 13:00, following the methods of Brandt et al. [19].
Supplied per kilogram of vitamin premix: 12,000,000 IU vitamin A, 2,400,000 IU vitamin D3, 132,000 IU vitamin E, 1,500 mg vitamin. K3, 3,000 mg vitamin B1, 11,250 mg vitamin B2, 3,000 mg vitamin B6, 45 mg vitamin B12, 36,000 mg pantothenic acid, 30,000 mg niacin, 600 mg biotin, 4,000 mg folic acid.
Supplied per kilogram of mineral premix: 80,000 mg Fe, 170 mg Co, 8,500 mg Cu, 25,000 mg Mn, 95,000 mg Zn, 140 mg I, 150 mg Se.
The presented numbers were calculated based on NRC [17].
The metabolizable energy (ME) was calculated based on NRC [17].
Based on AOAC [18] and HPLC.
Each sow’s body weight (BW) and backfat thickness were evaluated on d 112, at 24 h postpartum, and during weaning (d 133). The backfat thickness was also measured on the same days at 6.5 cm off the midline at the 10th rib using an ultrasonic device (Agroscan A16, Echo Control Medical). The leftover diets in the feeder troughs were collected to calculate average daily feed intake (ADFI) during lactation, farrowing, and at weaning to estrus intervals. Litter performance parameters, such as the number of piglets born, number born alive, number weaned (day 21 of lactation), survivability percentage, litter weight at birth, at weaning, as well as the piglet’s weight at birth and weaning, were recorded.
One week before weaning, chromium oxide (0.24%) was incorporated into the diet as a non-digestible inert marker. The diet was administered to all sows per replicate for 5 days, consisting of a 3-days adaptation phase followed by 2 days of sampling, preceding nutrient evaluation on d 133. Faecal samples were collected from each sow through gentle massage of the rectum. The harvested samples from each pen were pooled and then dried using a forced-air drying oven at 60°C for 72 h. The combined samples were subsequently milled using a Thomas Model 4 Wiley Mill (Thomas Scientific) with a 1-mm screen before being analyzed in triplicate for dry matter (DM) method 930.15, AOAC 2007, crude protein (CP) method 990.03, AOAC 2007, ether extract (EE) method 942.05, AOAC 2007, calcium method 985.01, AOAC 2007, phosphorus method 975.03, AOAC 2007, and acid detergent fiber method 973.18, AOAC 2007. Neutral detergent fiber content was determined by treating samples with amylase, sodium sulfite, and a neutral detergent solution. The resulting residues were filtered using a 1.5 μm glass fiber filter. The chromium (Cr) concentration was analyzed using an automated spectrophotometer (Jasco V-650, JASCO) following the method described by Fenton and Fenton [20]. Amino acid concentrations in feed samples were determined using high-performance liquid chromatography (HPLC; Agilent 1260 series, Agilent Technologies) following acid hydrolysis, with methodological modifications based on Hosseindoust et al. [21]. Organic matter was calculated by subtracting DM from ash content.
On the last day of the experiment (d 133), sows were given 1 mL of oxytocin (1 U/mL) to spur milk production. Fresh milk samples of 20 mL were then manually collected from the functional teats of all lactating sows in each replicate after wiping with alcohol ensuring no contamination from external sources. The samples were immediately transferred to sterile containers and stored at 4°C. Prior to analysis, each milk sample was thoroughly mixed to ensure homogeneity. A portion of the milk sample (typically 15 mL) was then transferred into the sample cup of the Milko Scan 133B Analyser (FOSS Electric). All samples were analyzed in duplicate to ensure accuracy and consistency of results. The MilkoScan 133B Analyzer was calibrated according to the manufacturer’s guidelines using the provided standard calibration solutions for fat, protein, lactose, total solids, and solids-not-fat. Regular calibration checks were performed to ensure the accuracy of the readings. The milk samples were placed in the sample chamber of the Analyzer which uses near-infrared spectroscopy for measuring the milk compositions. Each sample was measured individually, and the results were automatically recorded [22].
On d 133, 15 mL blood samples were collected from all sows via jugular vein puncture between 08:30 and 09:30 using K2 EDTA-coated vacutainer tubes (Becton Dickinson) to prevent clotting and minimize cytokine release from blood cells. Immediately after collection, the tubes were gently inverted 5–10 times to ensure proper mixing with the anticoagulant. Samples were then placed on ice and transported to the laboratory for further processing. To obtain plasma, blood samples were centrifuged at 3,000×g for 15 minutes at 4°C within 30 minutes of collection. Following centrifugation, the plasma was carefully pipetted into sterile microcentrifuge tubes, ensuring no disturbance of the buffy coat to prevent contamination with cellular components. Part of the plasma was used for evaluating tumour necrosis factor-alpha (TNF-α), Interleukin-10 (IL-10), and IL-1β determined using ELISA kits (MBS262753, MBS2513043, and MBS260684, MyBioSource) according to the manufacturer’s instructions. Part of the plasma was used for measuring total antioxidant capacity (TAC), superoxide dismutase (SOD), and malondialdehyde (MDA; MBS2611923, MBS265304 and MBS742540 MyBioSource). The remaining plasma was employed for evaluating zonulin and occluding, ELISA kits (MBS2607498, and MBS740246 MyBioSource) were considered following the manufacturer’s instructions. All the absorbance was measured at 450 nm using a microplate reader.
The method for measuring hair cortisol was outlined by Tajudeen et al. [23]. Briefly, freshly grown hair from individual sows was collected for cortisol analysis. Prior to this, a section of dorsal hair from the sows was removed at d 133. The hair samples were washed three times with isopropanol and then dried in a vacuum dryer at 35°C. They were then placed in an EML plastic tube containing steel pellets and processed using a bead beater (tacoTMPrep, 50/60 Hz 2A, GeneReach). Cortisol was extracted from the hair by methanol following crushing at the Biotechnology Corp, Taiwan. The cortisol concentration in the extracted samples was measured using an ELISA kit (ADI-900-071, Enzo Life Sciences).
We started by calibrating the pH meter (Sevenmulti, Mettler Toledo) using pH 4, 7, and 10 buffers, following the manufacturer’s instructions. The electrode was immersed in each buffer, allowing the meter to stabilize and adjust the readings accordingly. After calibration, the probe was rinsed with distilled water to avoid cross-contamination. Saliva samples were then collected from each sow using a sterile method (from the oral cavity) and transferred into clean containers. Briefly, the sow’s oral cavity was gently swabbed using a sterile cotton swab, ensuring that the swab did not contact external surfaces such as the snout or feeding trough to avoid contamination. The collected saliva was immediately transferred into sterile polypropylene tubes and sealed to prevent environmental exposure. All instruments and containers used were sterile and handled with disposable gloves to maintain sample integrity. The pH probe was submerged into the saliva sample for 20 seconds to allow the pH to stabilize, ensuring the probe was fully immersed but not in contact with the sides or bottom of the container. The displayed pH value on the meter was recorded after stabilization.
Faecal samples were obtained from all sows on lactation day 21 through rectal stimulation and promptly preserved at −20°C in sterile 50 mL conical tubes. Genomic DNA was isolated from 250 μL of each faecal sample using the QIAamp PowerFecal Pro DNA Kit (Qiagen), adhering to the manufacturer’s guidelines to maximize yield and minimize contamination. The extracted DNA samples were then stored at −20°C for subsequent analysis.
The V3–V4 hypervariable regions of the bacterial 16S rRNA gene were amplified using specific primers and processed for sequencing according to the standard Illumina 16S metagenomic library preparation protocol (Illuminav; Part No. 15044223 Rev. B). The resulting PCR amplicons were purified, adjusted to equimolar concentrations, pooled, and sequenced on an Illumina MiSeq platform using a 2 × 300 bp paired-end sequencing strategy.
Raw sequencing reads were assessed for quality, trimmed, and de-multiplexed using custom Perl scripts to enhance read accuracy and reduce sequencing artifacts. Processed sequences were analysed using Quantitative Insights into Microbial Ecology (QIIME2, version 2023.7). Amplicon sequence variants (ASVs) were identified through DADA2, and taxonomic classification was conducted using the SILVA 138-99 reference database. To account for variability in sequencing depth, a single rarefaction was applied to normalize ASVs to 18,911 reads per sample. This ensured unbiased comparisons across samples.
Alpha diversity metrics, including the Chao1 richness estimator and Shannon diversity index, were calculated in QIIME2. Beta diversity was assessed using Bray-Curtis dissimilarity, unweighted UniFrac, and weighted UniFrac distance metrics. Principal coordinate analysis (PCoA) was performed to visualize microbial community differences and was plotted using EMPeror software. Relative abundance at the phylum, family, and genus levels were analysed to assess microbiome composition. The differential abundance of bacterial taxa was evaluated using linear discriminant analysis effect size (LEfSe) to identify key microbial shifts [24,25].
Data were compiled in Excel and analyzed using a 2 × 2 factorial arrangement of treatments within a completely randomized design. The main effects of dietary feed forms, dEB levels, and their interaction were evaluated using the MIXED procedure in SAS (version 9.1; SAS Institute).
where Yijk is the observed response variable, μ is the overall mean, Ai is the fixed effect of feed form, Bj is the fixed effect of dEB level, (AB)ij is the interaction between feed form and dEB, Rk is the random effect of block (experimental week), and εijk is the residual error assumed to be normally distributed. Individual pigs were considered the experimental unit for all analyses.
Individual sows served as the experimental unit for all analyses. When data violated parametric assumptions, nonparametric analyses were performed using the Kruskal–Wallis test, with Bonferroni corrections applied to adjust for multiple comparisons and minimize type I errors. ASV features were statistically analysed using STAMP software (version 2.1.3, available at https://beikolab.cs.dal.ca/software/STAMP). β-diversity analysis was conducted through PCoA based on Bray–Curtis distance matrices to visually represent group differences. Microbial community structures were compared using permutational multivariate analysis of variance (PERMANOVA). Variations in individual ASVs across taxonomic levels were identified through pairwise Kruskal-Wallis H-tests in STAMP and visualized using graphical representations.
RESULTS
The effects of feed forms and dEB levels on sow performance are presented in Table 2. There were no significant differences in sow BW and backfat thickness during d 112, 24 h postpartum, and at weaning in all the dietary treatments. However, sows fed pellet feed forms Plow and Phigh, and higher dEB Mhigh and Phigh in diet had increased (p < 0.001) ADFI compared with Mlow.
The effects of feed forms and dEB levels on litter performance are presented in Table 3. There was no significant difference in litter size including total born, born alive, weaned, and survivability percentage. There was also no significant difference in litter weight at birth, at weaning, and piglet weight at birth. However, piglet weight at weaning was higher (p = 0.001) in Mhigh and Phigh compared with Mlow and Plow.
The effects of feed forms and dEB levels on nutrient digestibility and milk composition of sows are presented in Tables 4 and 5. The digestibility of DM was higher (p = 0.022) in feed forms Plow and Phigh compared with Mlow and Mhigh. There was no significant difference in CP and EE in all dietary treatments (Table 4). In Table 5, there was no significant difference in milk fat, protein, lactose, total solid, and solid not fat composition in all the dietary treatments.
The effects of feed forms and dEB levels on inflammatory cytokine and antioxidants of sows are presented in Tables 6 and 7. The TNF-α was lower (p < 0.001) in pellet feed forms Plow, Phigh, and higher dEB Mhigh and Phigh (p = 0.010), compared with Mlow, with significant interactions (p = 0.013) in feed forms and dEB. The IL-1β was lower (p < 0.001) in pellet feed forms Plow and Phigh compared with Mlow and Mhigh. There was no significant difference in IL-10 (Table 6). In Table 7, SOD was higher (p < 0.001) in pellet feed forms Plow and Phigh compared with Mlow and Mhigh. There was no significant difference in TAC and MDA in all dietary treatments.
The effects of feed forms and dEB levels on gut integrity, hair cortisol, and salivary pH of sows are presented in Tables 8, 9, and 10. There was no significant difference in the zonulin and occludin of sows (Table 8) in all treatments. In Table 9, the sow’s hair cortisol was lower (p = 0.048) in pellet feed forms Plow and Phigh compared with Mlow and Mhigh. In Table 10, there was no significant difference in salivary pH of sows in all dietary treatments.
| Feed form | Mash | Pellet | SEM | p-value | ||||
|---|---|---|---|---|---|---|---|---|
| dEB | Mlow | Mhigh | Plow | Phigh | Feed | dEB | Interaction | |
| Hair cortisol (pg/mg) | 165.71 | 161.32 | 154.67 | 151.85 | 7.08 | 0.048 | 0.013 | 0.090 |
| Feed form | Mash | Pellet | SEM | p-value | ||||
|---|---|---|---|---|---|---|---|---|
| dEB | Mlow | Mhigh | Plow | Phigh | Feed | dEB | Interaction | |
| Salivary pH | 7.46 | 7.47 | 7.48 | 7.48 | 0.02 | 0.669 | 0.974 | 0.767 |
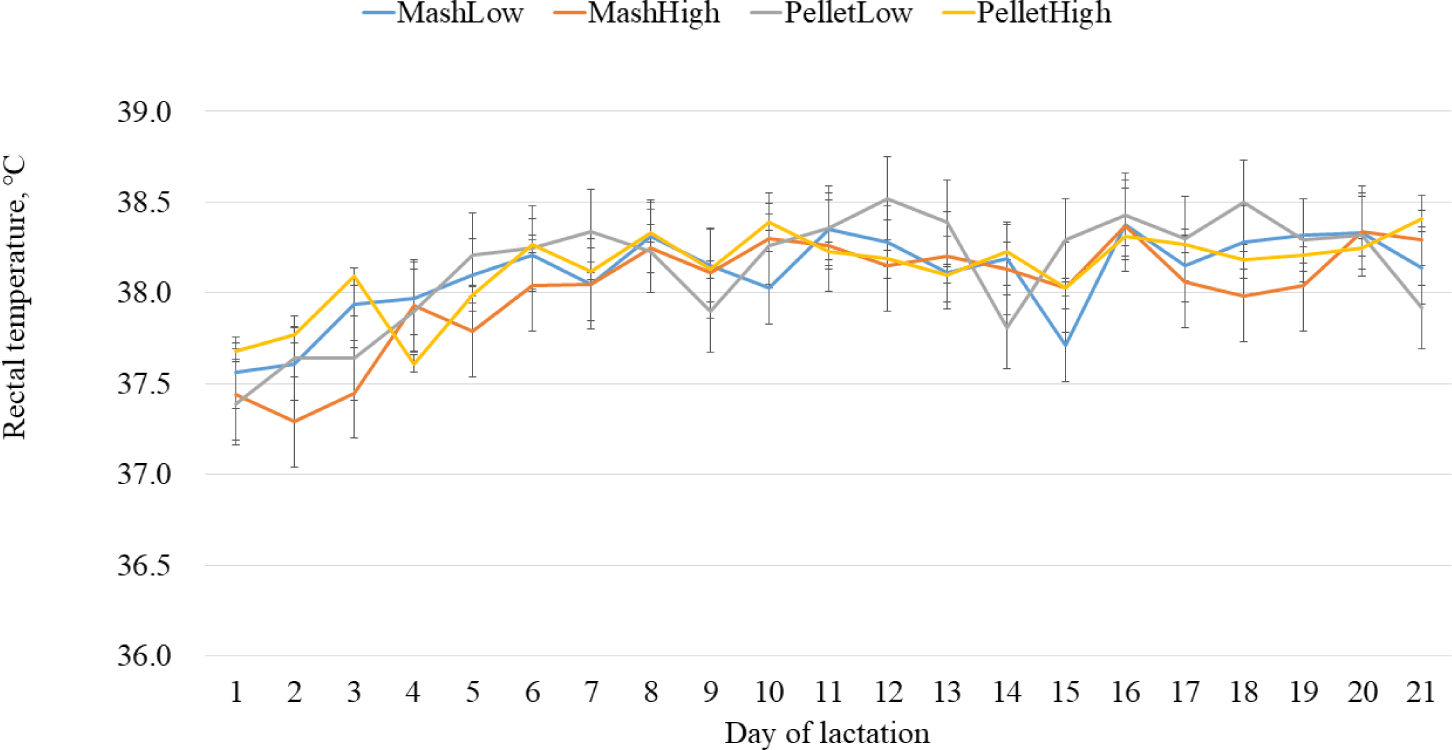
The ambient temperature (blue line) ranged from 26.0°C to 31.1°C with an average value of 28.8°C, while the THI (orange line) was below 70°C (Fig. 1). There was no significant difference in rectal temperature (Fig. 2), and respiratory rate (Fig. 3) throughout the experimental period.
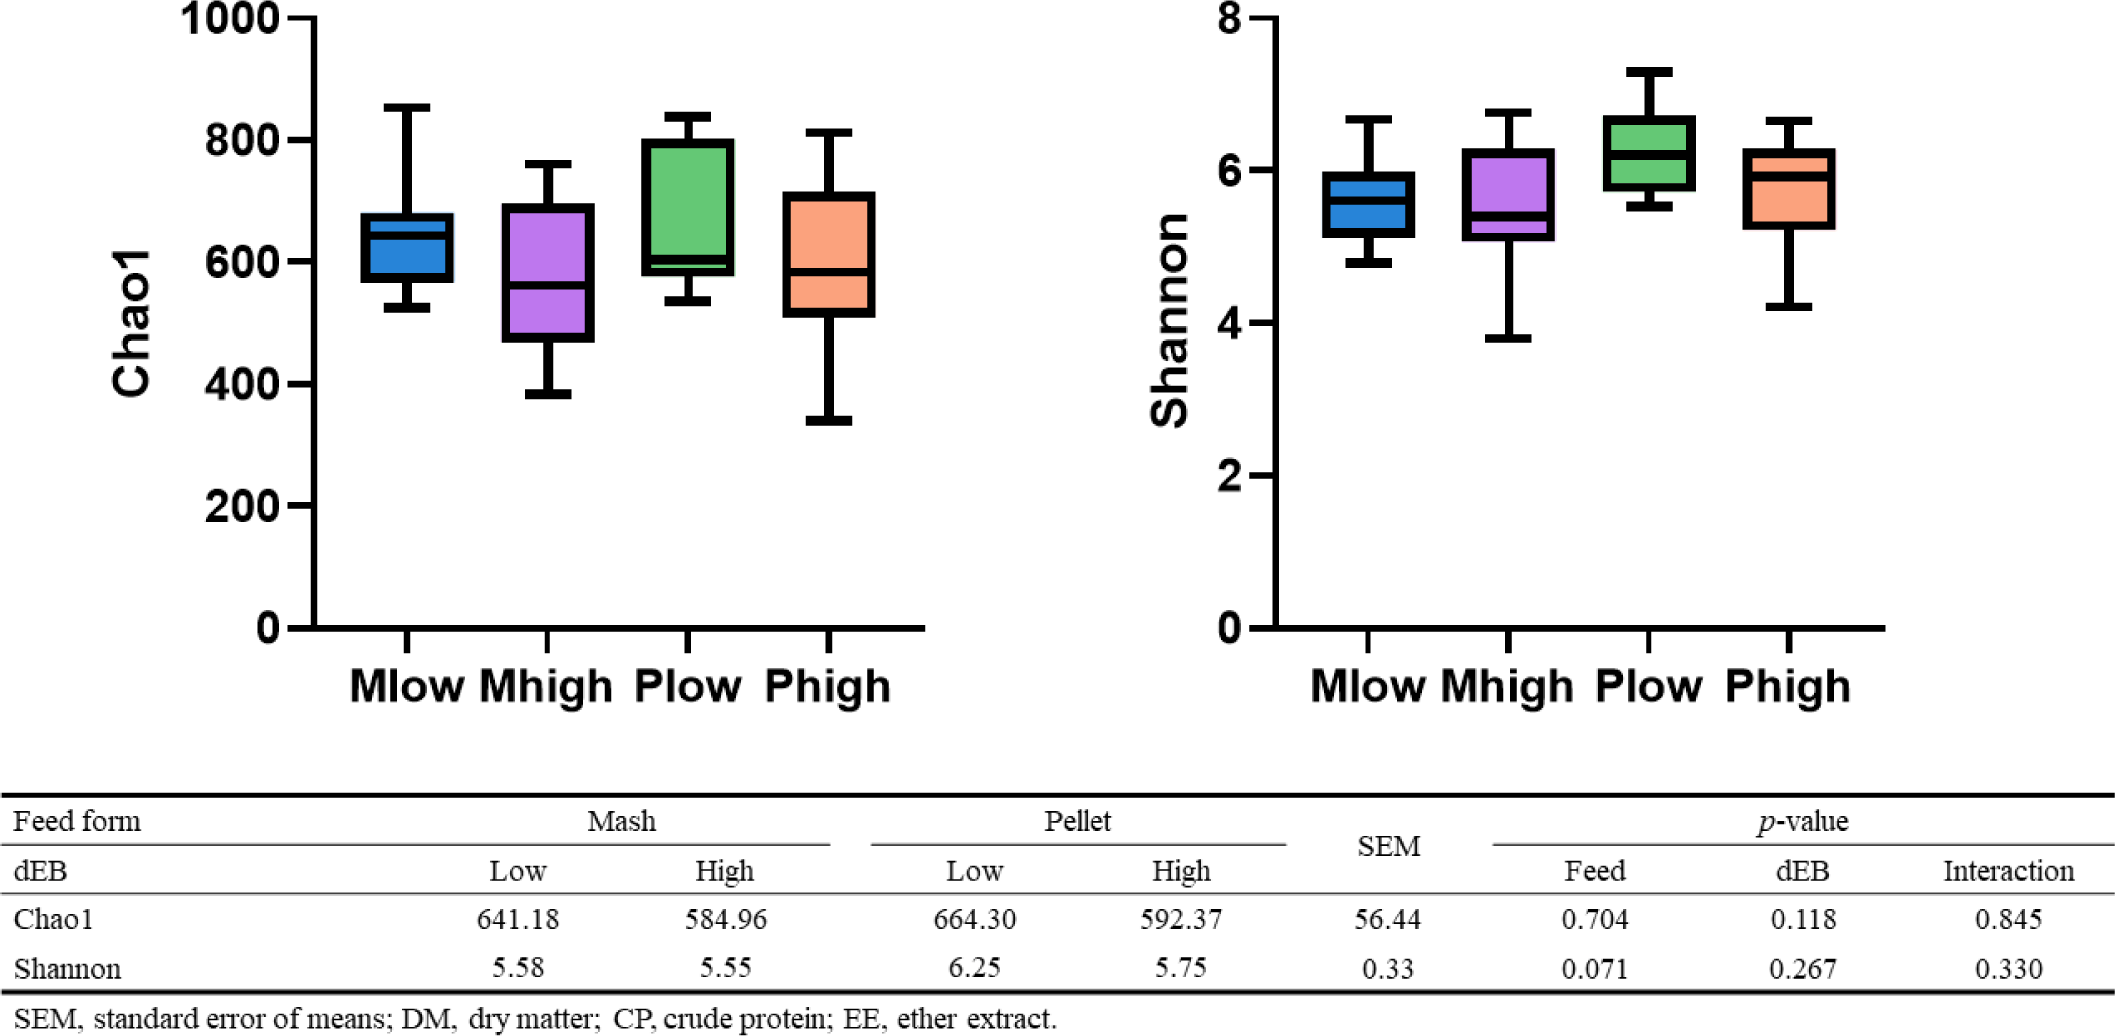
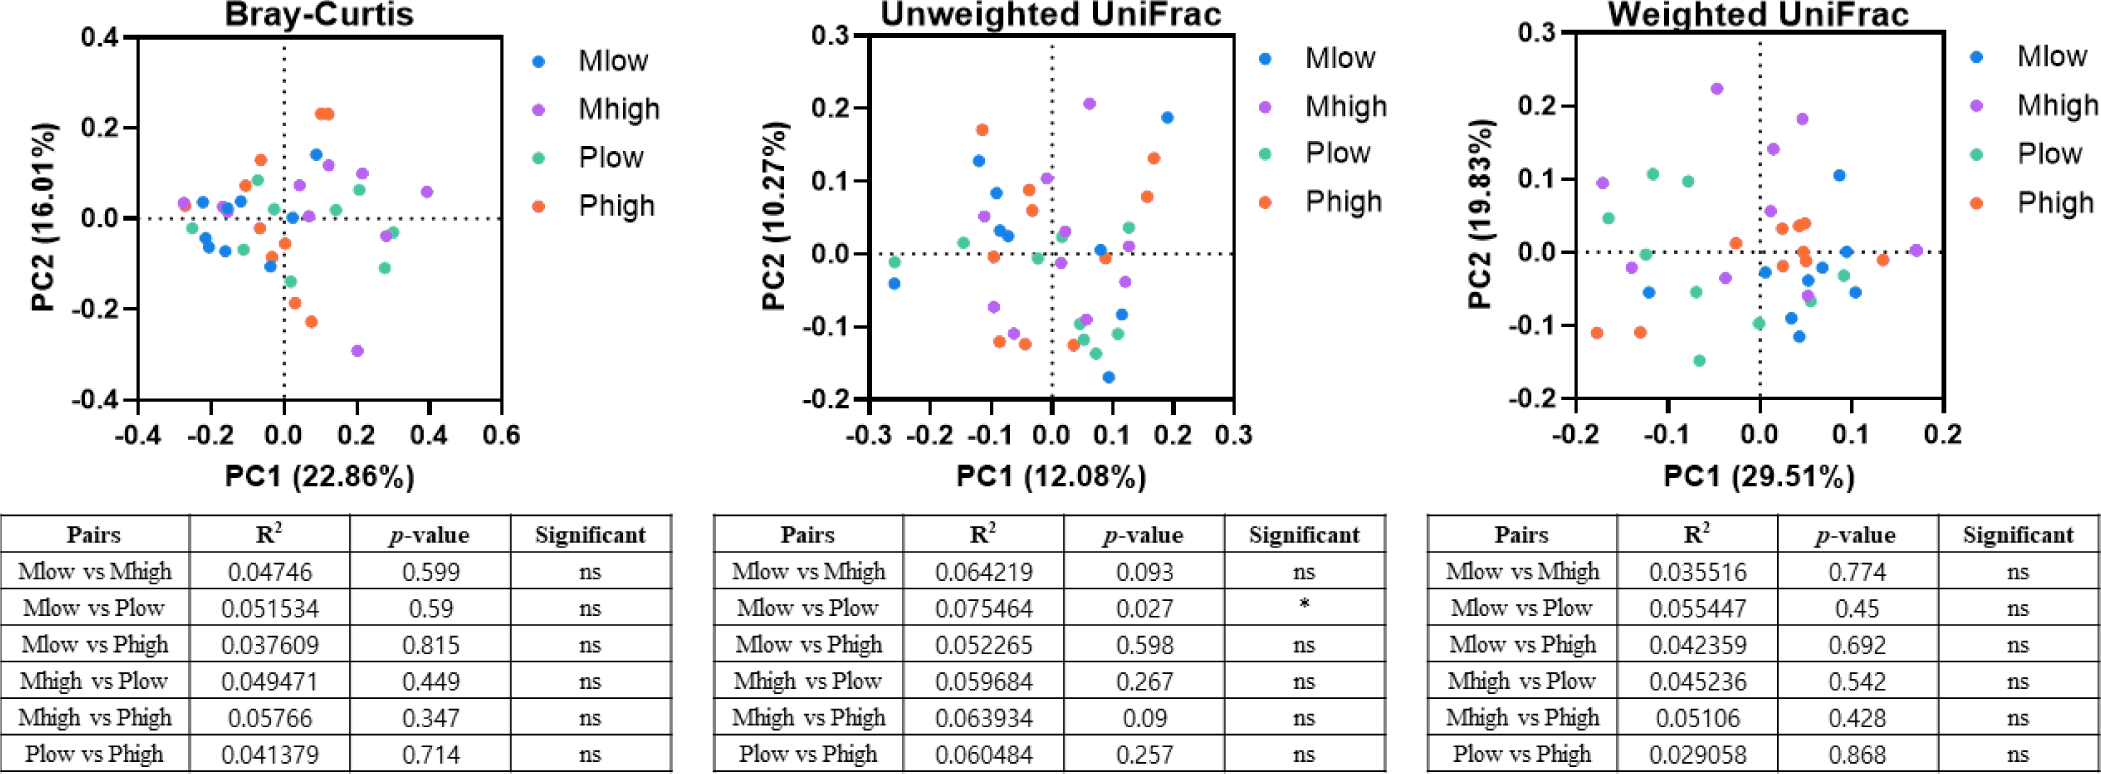
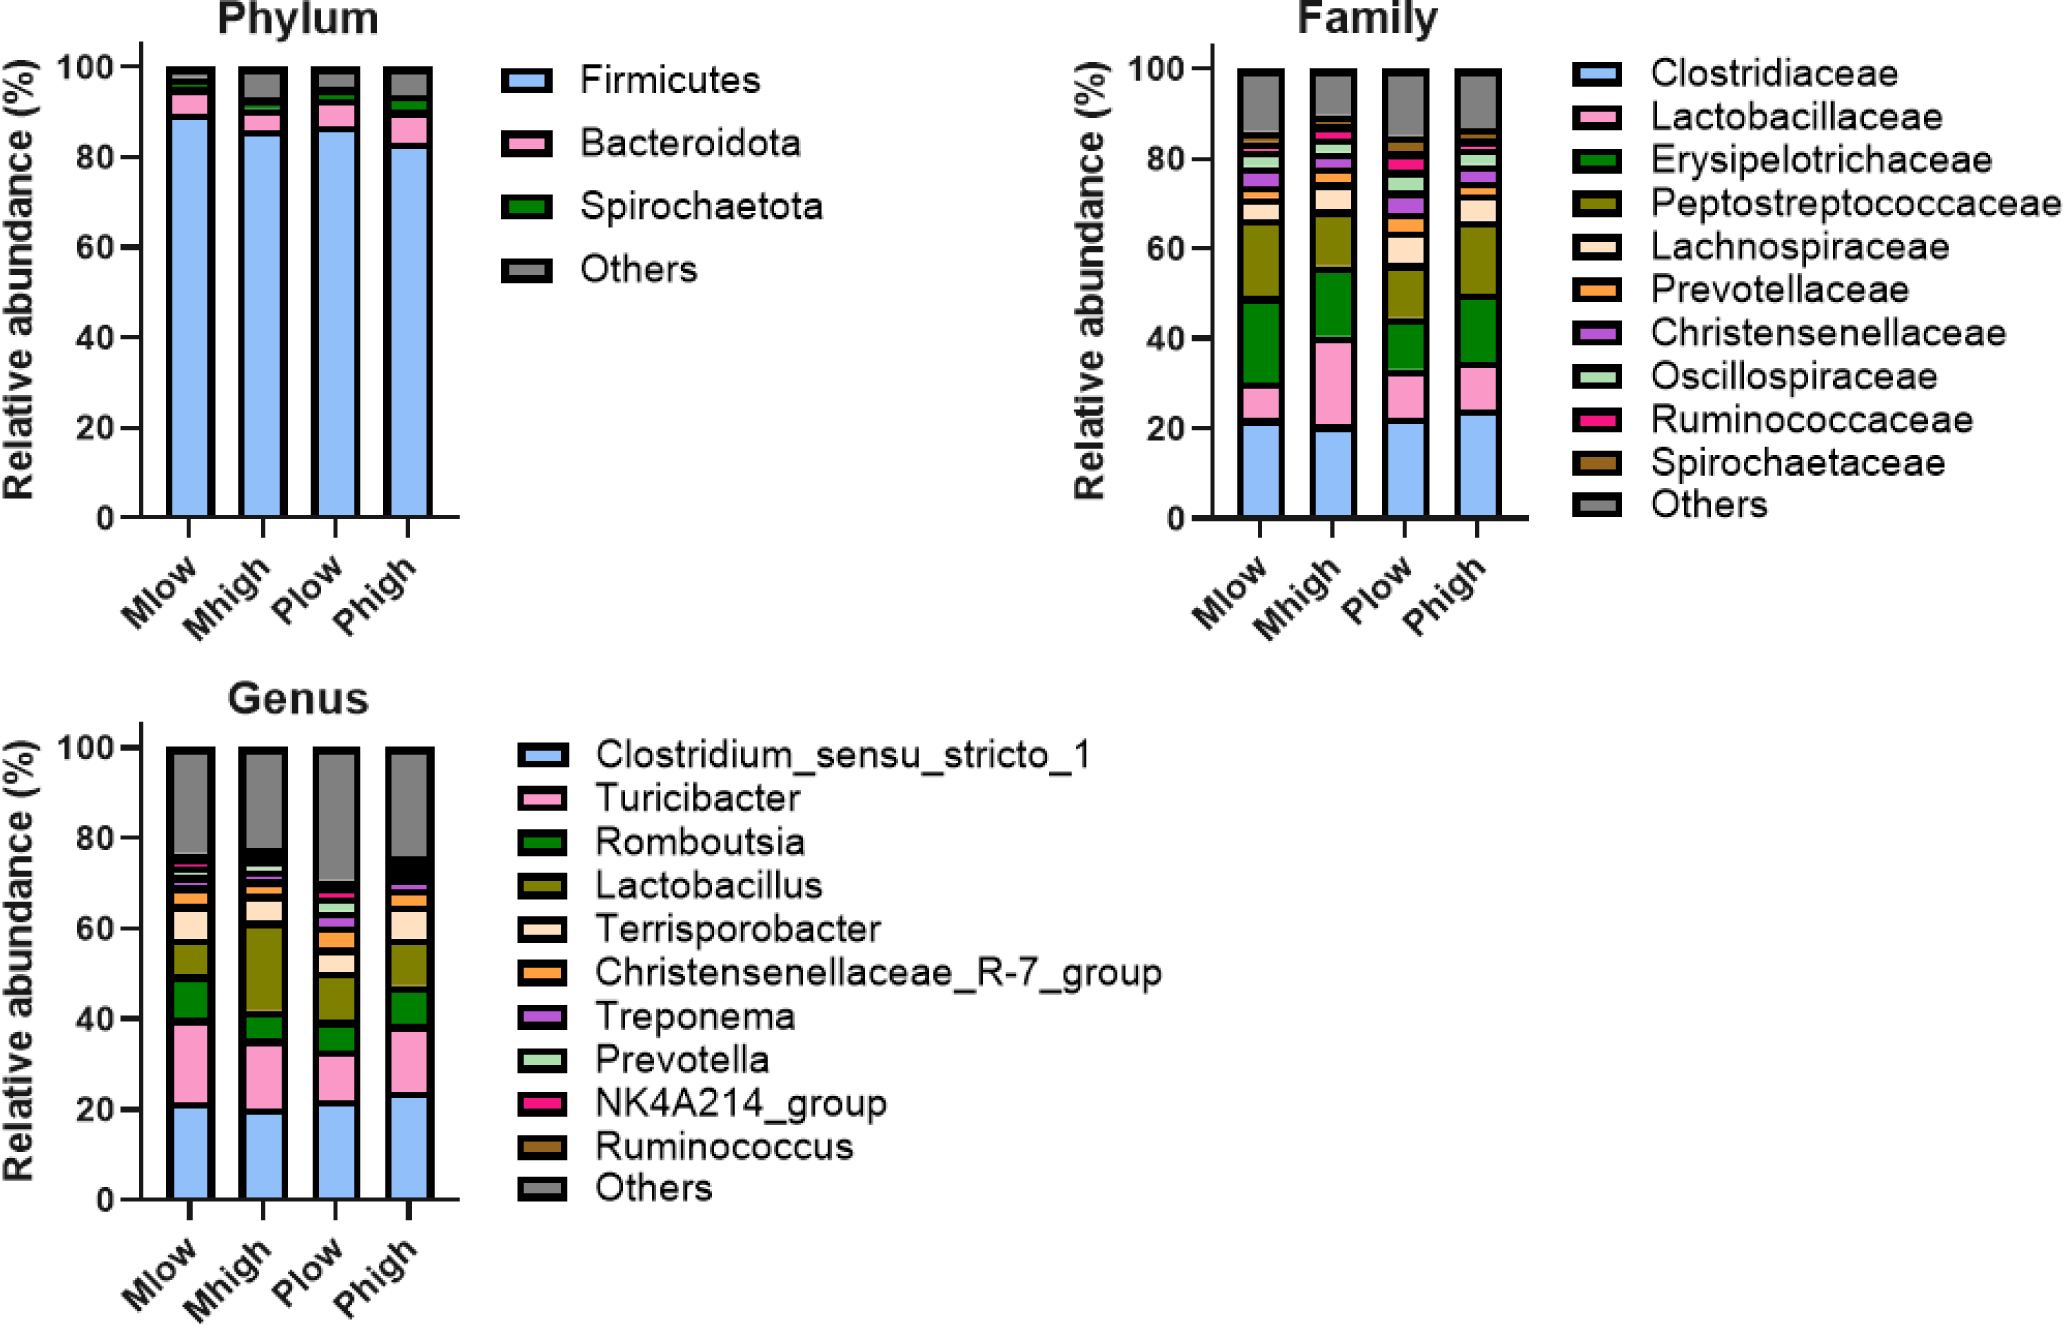
The effect of feed forms and dEB levels on alpha diversity (within-sample diversity) in lactating sows is shown in Fig. 4. There was no significant difference observed in Chao1 and Shannon in all treatments. In Fig. 5, there was a significant difference (p = 0.027) in Mlow vs Plow in the unweighted UniFrac (between-sample diversity). Lastly, as illustrated in Fig. 6, the relative abundance of microbial taxa in the phylum level showed no difference in Firmicutes, Bacteroidetes, and Spirochaetota. The microbial taxa at the family level showed higher Lactobacillaceae in Mhigh, while Phigh and Plow followed the same trend. Clostridiaceae, Erysipelotrichaceae, Peptostreptococcaceae, Lachnospiraceae, Prevotellaceae, Christensenellaceae, Oscillospiraceae, Ruminococcaceae, and Spirochaetaceae were not affected by the treatments. In the genus level, Lactobacillus was higher in Mhigh, with Phigh and Plow following the same trend. Turicibacter was higher in Mlow, while Prevotella was more obvious in Plow, and lower in Phigh, Mhigh, and Mlow. Clostridium, Romboutsia, Terrisporobacter, Christensenellaceae, Treponema, NK4A214 group, and Ruminococcus were not affected.
DISCUSSION
This study evaluated the effects of feed form and dEB levels on sow performance, immune status, gut health, and microbiota composition during lactation. While sow BW and backfat thickness remained unaffected, sows fed pelleted diets (Plow and Phigh) and those receiving higher dEB (Mhigh and Phigh) exhibited significantly greater ADFI, suggesting nutrient partitioning during lactation. Even though pelleted diets and higher dEB improved ADFI, the additional nutrients were likely directed toward sustaining milk production and supporting piglet growth rather than maternal tissue retention. Under HS conditions, sows mobilize body reserves to meet the high energy demands of lactation, and this metabolic prioritization often prevents detectable differences in body weight and backfat thickness despite higher feed intake [4,26,27]. Thus, the benefits of improved intake were manifested primarily in litter performance and physiological resilience rather than in maternal body condition. In addition, higher feed intake during lactation is important, as it directly influences maternal energy status and nutrient availability [22]. Consistent with improved maternal intake, piglets from the Mhigh and Phigh groups had significantly higher weaning weights, despite the indifferences in litter size or birth weights. This indicates that the elevated dEB in lactation diets may have enhanced nutrient transfer to offspring, potentially by improving nutrient absorption and flow [26]. Although milk composition (fat, protein, lactose, and solids) did not differ among treatments, greater DM digestibility was observed in sows fed pelleted diets (Plow and Phigh), which may explain the improved growth performance of piglets. The improved nutrient digestibility likely enhanced the efficiency of nutrient transfer to offspring during lactation. Feed form is known to influence nutrient utilization, with pelleted diets often enhancing nutrient availability through reduced sorting and improved digestibility [10]. The lack of variation in milk composition suggests that while feed form and dEB levels may influence the quantity of milk or its physiological impact as reflected in piglet growth, they do not significantly alter its nutritional profile. Such stability in milk composition is beneficial, as it ensures that piglets receive consistent nutrient profiles during the suckling phase, regardless of maternal dietary modifications. Taken together, our findings indicate that both feed form (pelleting) and higher dEB effectively improved sow performance and feed intake under HS. The tendency for interactive effects on ADFI and piglet weaning weight highlights the potential benefits of combining pelleted diets with higher dEB.
The immune-modulating effects of the dietary interventions were demonstrated by the reduced levels of pro-inflammatory cytokines TNF-α and IL-1β in sows fed pelleted diets and those receiving higher dEB. As key mediators of inflammation, the downregulation of these cytokines is typically linked to a more regulated immune response, improved gut integrity, and reduced oxidative stress [28,29]. These effects may be attributed to the combined physiological benefits of pellet processing and electrolyte balance. High dEB diets enhance systemic buffering capacity, potentially reducing gastric acidity that protects the non-glandular region of the stomach, where ulcers commonly occur [15,16,30]. Concurrently, pelleted diets promote consistent feed intake and uniform gastric emptying, helping to minimize fermentation-induced acid accumulation and mucosal irritation [9,10]. Such anti-inflammatory state may support improved nutrient absorption and productivity during the metabolically demanding HS and lactation period. This is further supported by increased SOD activity in sows fed pelleted diets, indicating enhanced antioxidant defense. Moreover, the significant interaction observed for TNF-α suggests a synergistic effect when pelleted feed is combined with higher dEB.
Although markers of gut barrier integrity (zonulin and occludin) were not significantly affected, sows fed pelleted diets had lower hair cortisol concentrations, which may reflect reduced chronic stress during lactation. Our findings align with improved feed intake and inflammatory status in pelted feed which could have practical implications for sow welfare [31]. While direct studies on pelleted feed reducing stress in lactating sows are limited, it is recognized that improved feed intake and nutrient digestibility can alleviate metabolic stress [27]. Enhanced nutrient absorption supports better energy balance, which may contribute to reduced physiological stress responses [32,33]. For lactating sows, a THI value below 72 is generally considered thermoneutral, 72–78 indicates mild heat stress, 79–88 indicates moderate stress, and values above 88 indicate severe stress [19]. During the experimental period, the THI ranged from 75.58 to 82.76, which corresponds to mild to moderate heat stress conditions. Salivary pH and physiological heat stress indicators (rectal temperature and respiratory rate) did not differ between treatments, and the ambient THI remained within the thermoneutral range, indicating that environmental heat load was unlikely to confound treatment effects. The tendency for interactive effects observed in hair cortisol further indicates a synergistic benefit of combining pelleted feed with higher dEB.
Microbial diversity is a crucial aspect of animal nutrition as it is linked to better overall health, including nutrient absorption, immune function, and disease prevention [34]. Our microbial diversity analysis revealed no significant differences in alpha diversity across treatments, suggesting that microbial richness and evenness were maintained. However, beta diversity analysis (unweighted UniFrac) revealed distinct microbial compositions between Mlow and Plow, suggesting that feed form influenced microbial structure even in the absence of major diversity shifts. At the family and genus levels, the relative abundance of Lactobacillaceae and Lactobacillus was higher in Mhigh, with similar trends in Phigh and Plow, possibly contributing to improved gut health and anti-inflammatory responses [35]. Turicibacter, which has been associated with immune activation and oxidative stress [36,37], was elevated in Mlow, aligning with higher inflammatory markers in this group. Conversely, Prevotella was most abundant in Plow, a genus often linked to fiber fermentation and carbohydrate metabolism [38], although its role is context-dependent and requires species-level interpretation.
In conclusion, these findings suggest that the interaction between pelleted feed form and higher dEB levels (Phigh) emerged as the most effective result during lactation by improving feed intake, litter performance, anti-inflammatory responses, antioxidant status, and influence gut microbial composition without negatively impacting milk composition or gut integrity. These outcomes support the use of pellet processing and high dEB as complementary strategies to enhance sow productivity and health in lactation period during heat stress.


